


“ All Life is Problem Solving” - Karl Popper (Popper, 1999)
You don’t need a brain to have a mind.
That sounds like a provocation, but it may also be the beginning of a new way of understanding mind and life.
For the last century, we have been taught to think of cognition as something brains do. Neurons fire, networks compute, thoughts emerge. That picture has been enormously powerful, but what if it is also too narrow?
Cells are not passive bags of chemistry. A single cell senses, evaluates, repairs, remembers, moves, metabolizes, and survives in a turbulent world. A bacterium compares past and present chemical conditions as it swims toward food. A slime mold solves mazes without a nervous system. A ciliate, faced with irritation, tries one response, then another, as if working through a tiny behavioral repertoire.
Welcome to Cellosophy: our attempt to understand cognition from the bottom up, beginning not with the human brain but with the living cell. In the essay below, we invite you into a new scientific adventure: to look through the microscope not only for the machinery of life, but for the primordial origins of mind. Follow along as we explore the possibility that intelligence is as ancient as life itself.
Introduction
Cognition has puzzled philosophers and scientists for centuries, but the last hundred years have arguably seen more progress than the previous three thousand. The modern approach is made possible by the remarkable synthesis of two major breakthroughs, one experimental and one conceptual: on the one hand Ramon y Cajal’s discovery that the messy spaghetti of the brain is in fact an orderly network of individual cells communicating electrochemically (Cajal, 1906) and on the other the invention of the computer in the 1930s - not merely a faster calculator, but, in Turing’s formulation, a universal machine capable of carrying out any effective computation that can be carried out at all (Turing, 1937).
The fertile intersection of these two innovations made scientists confident that for the first time, we had a concrete and process-oriented understanding of how the mind works: it is a vast network of individual cells, each making a minuscule contribution to refining a stream of information, culminating eventually in intelligent thought.
In 1943, McCulloch and Pitts gave this intuition a precise mathematical form: a neuron with multiple inputs, logical thresholds, and a single all-or-none output (McCulloch and Pitts, 1943). It was elegant, scalable. Rosenblatt’s perceptron soon turned the idea into a trainable unit of pattern recognition, the ancestor of artificial neural networks and the conceptual foundation of today’s explosion in statistical artificial intelligence (Rosenblatt 1958). You have to appreciate the power of this fundamental synthesis of biology and computational logic. It allows us to formulate and answer so many questions that it fully deserves to be treated like a sacred cow.
We have long known that neurons are more complex than switches, but of late, it’s becoming clearer that the complexity matters for cognition. Dendrites - the putative weighted receptors of incoming signals - turn out to have active branching neighborhoods, performing nonlinear integration, generating local spikes, and in human cortical neurons even supporting computations classically associated with multilayer networks ( Stuart and Spruston, 2015; Gidon et. al, 2020). One recent modeling study found that reproducing the input-output behavior of a single cortical pyramidal neuron required the equivalent of a five-to-eight-layer artificial neural network (Beniaguev et. al., 2021). Fried and colleagues’ famous single-neuron recordings in epileptic patients revealed “concept cells” or “grandmother” neurons: cells that respond selectively to strikingly different images of the same person, landmark, or object, and sometimes even to written names (Quiroga et. al., 2005). Of course, when pressed, systems neuroscientists or cognitive neuroscientists will agree that neurons are more complex, but then: does this additional complexity matter when it comes to analysing human (or mammalian) behaviors? One way to explore that question is by studying biological systems that don’t number in the thousands or millions of cells.
What if we study biological systems at the other end of multicellularity from creatures that possess nervous systems, namely, unicellular creatures? Any behavioral complexity they possess must be due to capacities of a single cell, not that of a collection.
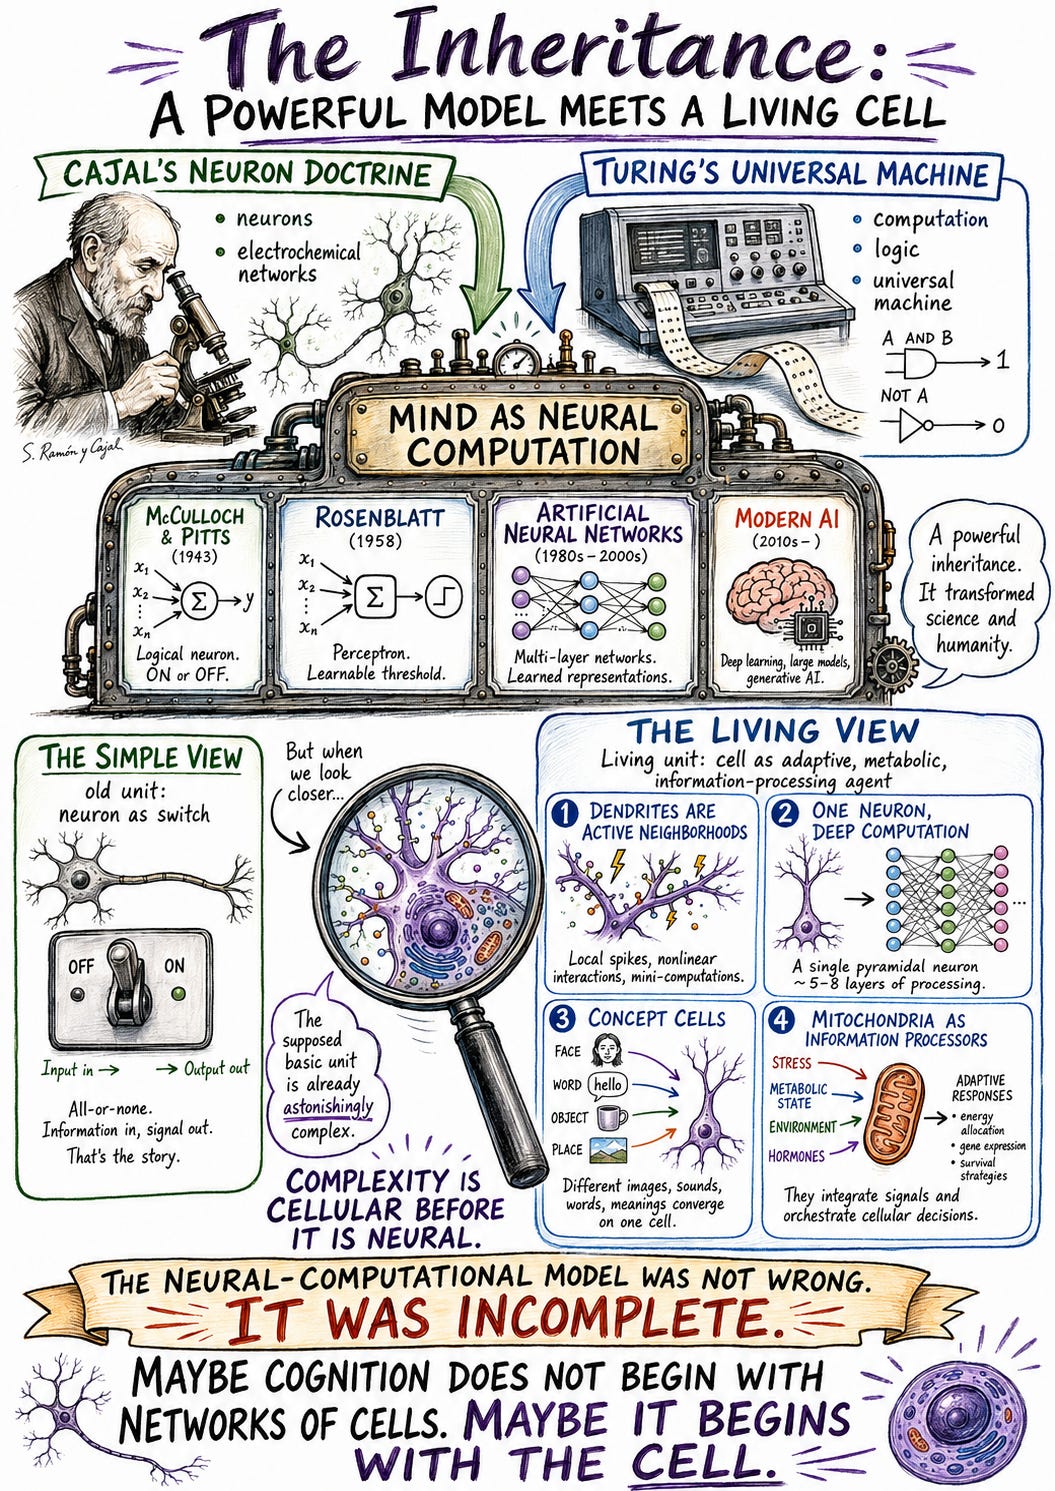
As we began exploring this idea, we started looking for cases of behavioral adaptability. Mitochondria, for instance, are not merely the cell’s power plants. Many nucleated cells, including neurons, contain hundreds to thousands of mitochondria, and these organelles continuously remodel themselves in response to cellular demand (Picard and McEwen, 2018). In their recent synthesis “Mitochondrial signal transduction,” Picard and Shirihai argue that mitochondria sense, integrate, and transduce biochemical, metabolic, environmental, and neuroendocrine inputs into adaptive cellular and organismal outputs. They call this distributed organelle-level architecture the Mitochondrial Information Processing System, or MIPS (Picard and Shirihai, 2022).
Signal transduction is a rather complex affair at the scale of a single cell. Perhaps the brain isn’t an intelligent aggregate of dumb parts, but rather a society of already-competent living cells, coordinated into higher-order dynamics. This recasts the question of cognition: what if the mind is anchored in the architecture of the single cell?
Evidence for this alternative vision has been accumulating, but unfolding it involves in some sense a costly transition: it requires a fundamental rethink of our understanding of the nature of cognition. We invite you to participate in exploring and charting this new territory. This investigation will impact our understanding of our own minds, the processes taking place within individual cells, and the models we can develop for artificial cognition. It will require the cooperation of researchers in multiple disciplines.
Yet the initial focal point is simple: the nature of the individual cell, the behaviors that demonstrate cognition, and the processes that make it possible.
By returning to the biological basics, we can trace the evolutionary continuity of the mind, understand the intimate link between a cell’s internal metabolic demands and its external environment, and potentially use cognition as a universal lens to view all living systems. Through this reframing, Cellosophy aims to not only explore the origins of cognition but to challenge our assumptions about the future of artificial intelligence and, perhaps, the nature of life itself.
The Evolutionary Continuity of Cognition
The first, and perhaps most intuitive, reason to study the cognitive capacities of single-celled organisms is to treat cognition exactly like any other evolved characteristic of animals.
In evolutionary biology, we do not expect animal metabolism to have evolved entirely separately from the metabolism of other, simpler creatures. There are mitochondria in most eukaryotic cells, utilizing ancient, conserved biochemical pathways to generate ATP. In the very same way, could cognition in its rudimentary forms be present even in unicellular organisms? The way these microscopic entities sense and react to their environments provides vital clues about the origins of cognition itself. This biogenic approach, often referred to as “basal cognition” (Lyon and Cheng, 2023) - serves as the baseline for the emergence of all intelligence in the biosphere.
Solving Slime Molds and Decisive Ciliates
When we look closely at the behavior of unicellular eukaryotes, we find remarkable evidence of what we would readily call cognitive behavior if it were observed in creatures like us. We know that single-cell organisms are capable of highly sophisticated actions.
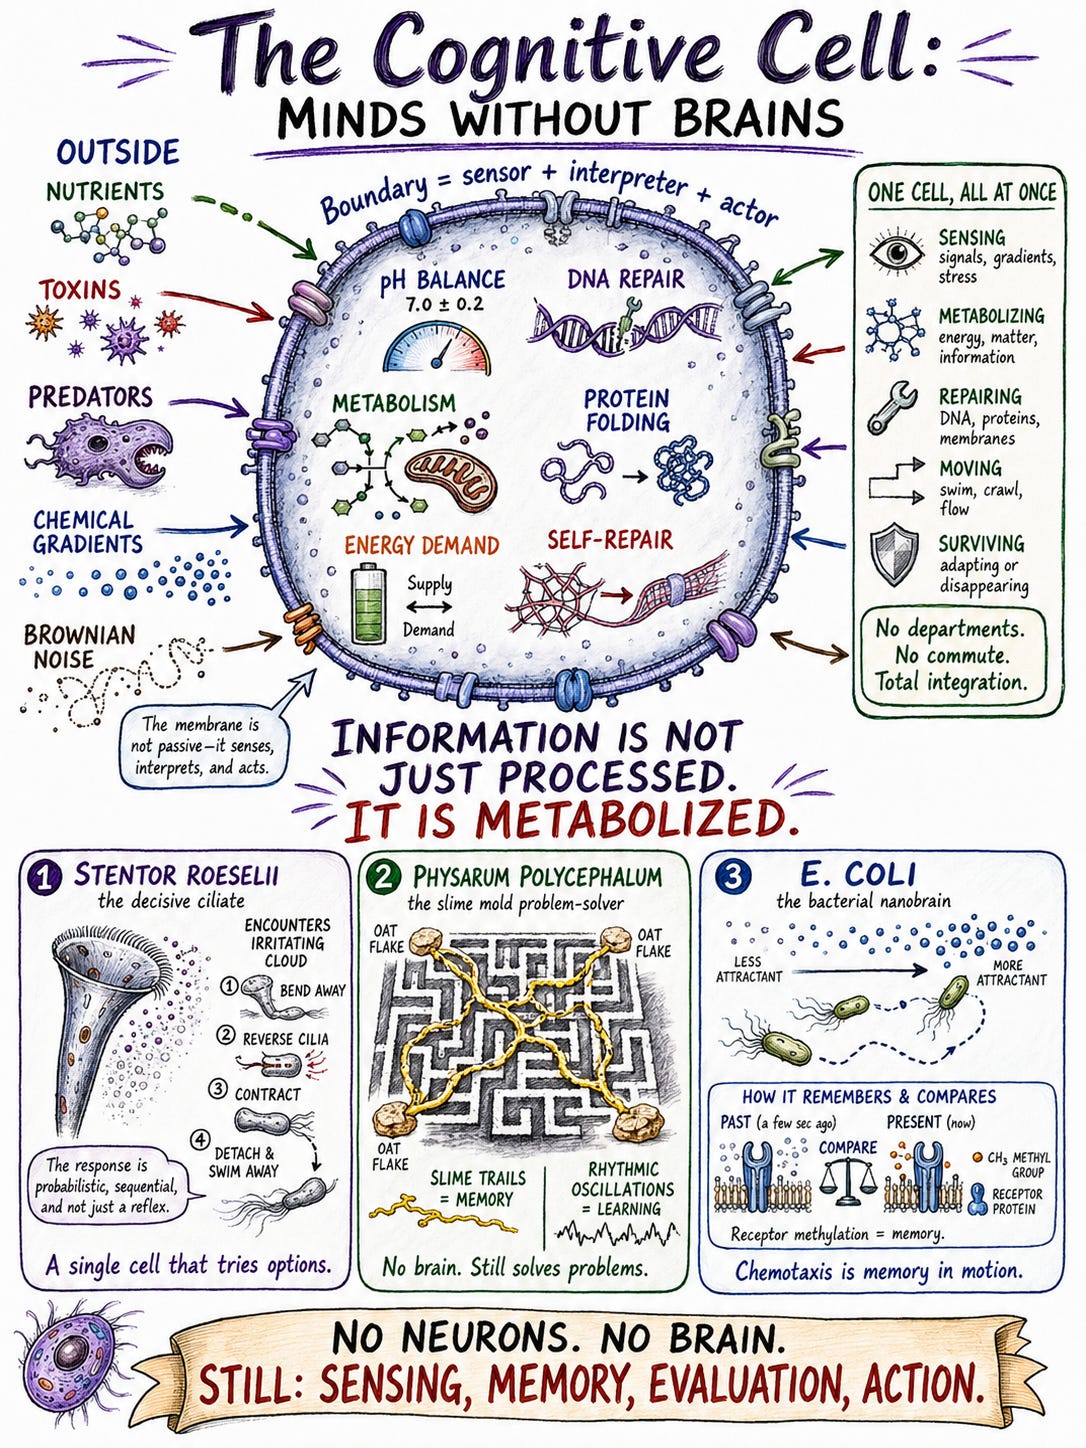
Consider the giant, single-celled ciliate Stentor roeselii. Over a century ago, the pioneering zoologist H.S. Jennings observed (Jennings, 1906) that this trumpet-shaped organism does not merely react reflexively to an irritating stimulus, like a cloud of carmine dye. Instead, it exhibits a complex behavioral hierarchy. Recent replications of this work by modern systems biologists, such as Jeremy Gunawardena and Joseph P. Dexter, have confirmed (Dexter et. al., 2019) that when faced with a persistent threat, Stentor can respond in one of several ways: bend away, reverse its ciliary beating, contract, or detach and swim away. Incredibly, the response is not deterministic, but probabilistic. The cell seemingly “changes its mind,” demonstrating sequential logic, habituation, and a foundational form of decision-making.
Similarly, the acellular slime mold Physarum polycephalum has shattered assumptions about the necessity of a brain for complex problem-solving (Nakagaki et. al., 2000). Research by several groups has shown that this sprawling, single-celled (but multinucleate) amoeboid organism can solve the famous “Traveling Salesperson Problem” (Zhu et. al., 2018), navigating mazes to find the shortest path between food sources. It utilizes a form of spatial memory encoded in the extracellular slime trail it leaves behind, and it even demonstrates economically ‘irrational’ choices based on past experiences and heuristic evaluations of risk. The slime mold retains information and learns through rhythmic biological oscillations.
The Bacterial “Nanobrain”
This cognitive toolkit extends all the way down to prokaryotes. As the philosopher Pamela Lyon (and in a different vein, Levin and Dennett) has extensively argued, perhaps all living cells are cognitive (Lyon & Cheng, 2023; Levin and Dennett, 2025). Bacteria such as Escherichia coli and Bacillus subtilis display profound abilities to process information. Bacterial chemotaxis, i.e., the process by which a bacterium navigates chemical gradients, is not a blind physical reaction but a sophisticated computation. The bacterium utilizes an internal working memory, relying on receptor methylation to compare the concentration of nutrients in its past with its present, allowing it to navigate toward a better future.
In light of this, it is time to seriously consider unicellular organisms as cognitive creatures in their own right. We must study the rudimentary forms of cognition that these organisms possess.
Blurring the Boundary Between Inside and Out
The second primary reason to study cognition at the cellular level is that in unicellular organisms, information processing is inextricably tied to other processes that solve the organism’s existential needs: metabolism, autopoiesis (self-creation), and homeostasis. In complex animals, the nervous system acts as a specialized buffer, processing external stimuli at a safe distance from the core metabolic functions of the gut or the liver. But in a single cell, there is no such luxury of distance. What it takes for a unicellular organism to maintain its structural integrity is intimately and immediately related to how that organism senses its environment.
Put another way, the sensory world of animals like us is dominated by entities approximately their size such as predators/prey or rocks to navigate around. In contrast, their interior environment has threats such as infection that are orders of magnitude smaller such as viruses. There’s a strong asymmetry between inside and outside, so to speak. In contrast, for a bacterium, the predator (such as a white blood cell) is approximately the same size as cellular processes that guide growth and reproduction. Inner and outer are a lot closer in size. Chemistry matters on both sides; random noise matters on both sides.
Navigating an Uncertain Micro-World
To understand this, we must consider the physical reality of the single cell. At the microscopic scale, cells exist in a low-Reynolds-number environment dominated by viscous forces and the relentless, chaotic bombardment of Brownian motion.
Because of this reality, the gap between the physics of the ‘outside’ and the ‘inside’ is considerably less pronounced than it is for multicellular creatures. The cell’s boundary is not just a wall; it is a highly dynamic sensory organ. Theorists like František Baluška have conceptualized this as the ‘Senome’: the sum of all sensory experiences and apparatuses of the cognitive cell (Baluška, 2025). Because the internal and external physical (fluid) environments are similar, physiology and cognition are fundamentally fused.
Problem-Solving Across the Spectrum
Because of this fusion, we can understand how information is utilized simultaneously for both the interior and exterior needs of the organism. This leads to the formulation of overlapping problems that the organism must solve.
More generally, the nature of the problems that a unicellular organism has to solve to meet its internal demands (such as regulating gene expression, repairing DNA, and maintaining pH balance) are closely related to the problems it solves to meet its external demands (such as finding food, evading toxins, and communicating with kin). For creatures like us, deciding what to eat and the biochemical process of digesting that food may feel entirely separate, but are they? For a bacterium or an amoeba, the distinction between metabolism and cognition may be impossible to draw; these are continuous phenomena along an internal-external spectrum. The cell is continuously responsive to the confluence of internal and external factors, generating highly information-dense decisions that cannot be understood as uniquely “material” or “cognitive”.
Are Cells thinking matter? (Ramanathan and Broach, 2007)
From the perspective of enactivism and cybernetics, cognition is not an abstract processing of symbols, but the very activity of a living system maintaining itself in relation to its environment (Maturana and Varela 2012). Therefore, the continuous nature of problem-solving needed for a unicellular organism to survive provides a model for how biological computation actually works. Information is not just processed; it is metabolized. Memory and learning are not just mental states; they are physical configurations of the cytoskeleton, epigenetic states of the organism, and the dynamic biochemical networks of the cell.
The Cognitive Lens on Life
This seamless continuity brings us to the third overarching possibility of Cellosophy: that cognition is not merely an isolated phenomenon to be studied, but a universal biological capacity (Lyon, 2015; Levin and Dennett, 2025). Cognition serves as a powerful conceptual lens through which we can observe and understand what a living being does (Thompson, 2010). Thinking of life as ‘code’ has been enormously productive (and reductive...); can cognition play a similar role?
Cognitive processes are not reserved solely for sensing the external environment. They are actively deployed for metabolizing energy sources and keeping the interior environment within the strict, life-sustaining parameters of homeostasis. When we recognize this, the definition of cognition shifts from “thinking” in the anthropomorphic sense to a broader, heterarchical control mechanism that allows any autonomous living entity to navigate uncertainty.
> Of course, this shift in our framing of cognition can also mean it is reducible to the (purely physical) dynamics of complex, hierarchical systems, but that would be good to know, wouldn’t it?
Multicellularity as a Cognitive Solution
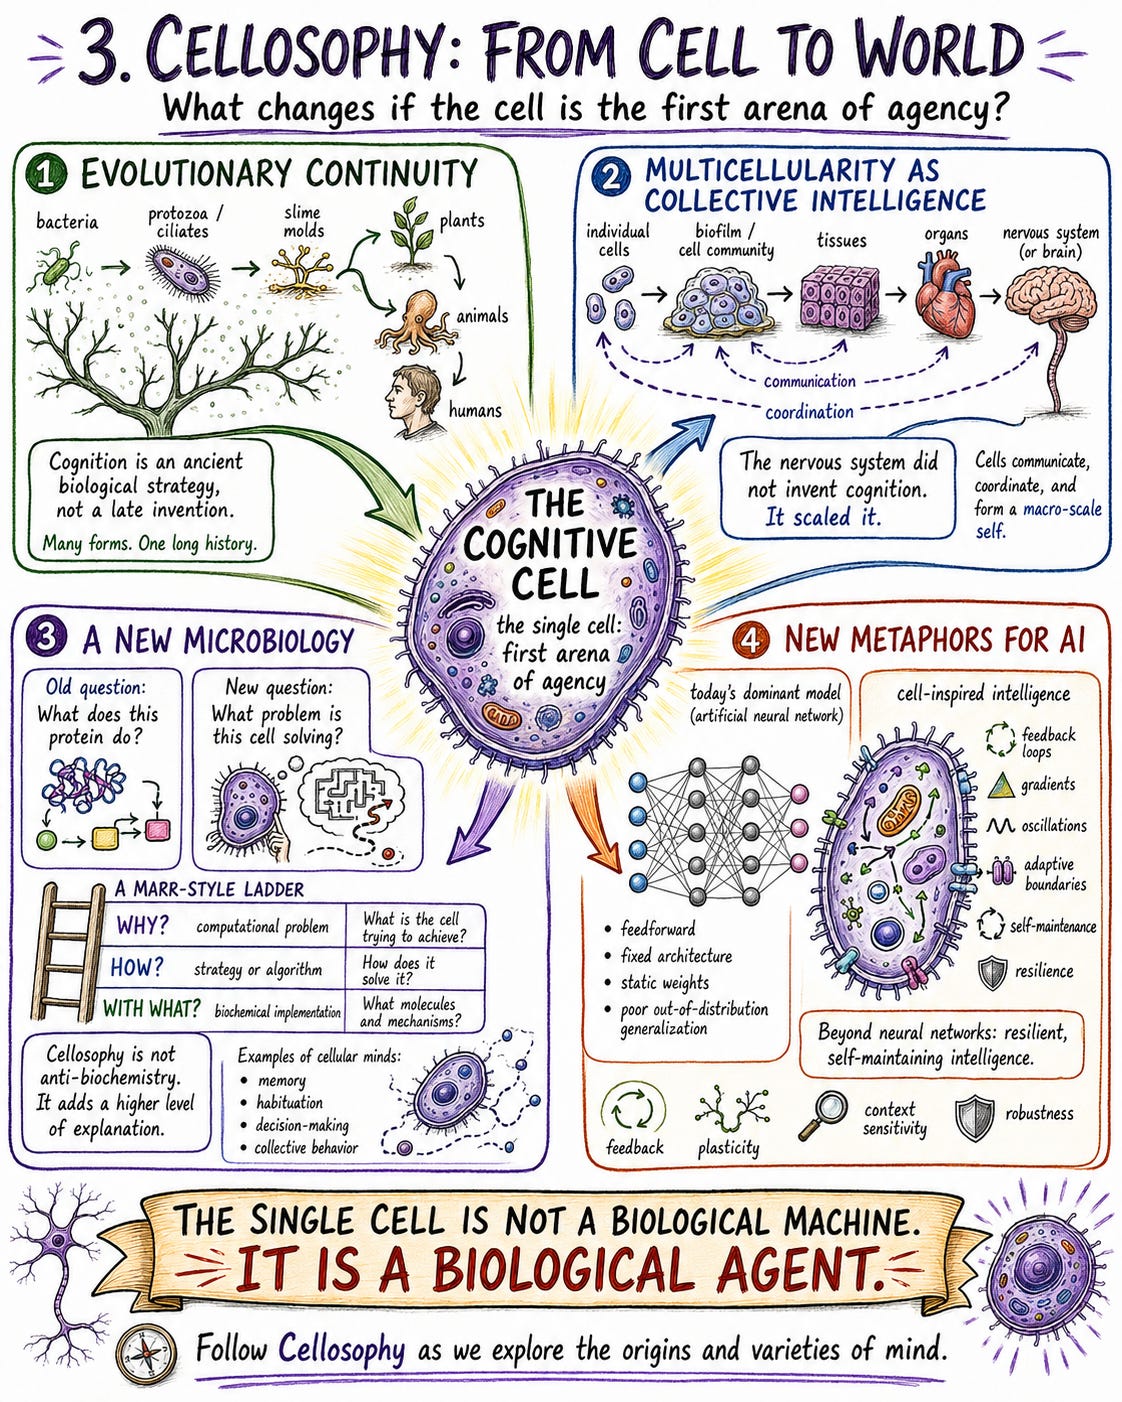
If we view all cellular activity through this cognitive lens, major evolutionary milestones take on a radically new light. It may be that the transition from unicellularity to multicellularity itself - not the dominant choice, since two of the three kingdoms and most phyla remain unicellular - was fundamentally a cognition-like solution to a computational problem. In this picture, multicellularity is one way to explore the space of all possible minds, though the investment in expensive ‘hardware’ both helps multicellular organisms explore regions of possibility space that might otherwise be inaccessible, but also makes them resource hungry and potentially fragile. Dinosaurs and humans will come and go, but bacteria will be around as long as the sun permits them to do so; a red giant sun will likely kill them off too.
When single cells aggregate, as seen in bacterial biofilms, social amoebae like Dictyostelium, or the early ancestors of plants and animals, they must solve profound challenges of collective action, resource sharing, and spatial organization. As theorists Argyris Arnellos and Alvaro Moreno have argued (Arnellos and Moreno, 2016), multicellular organisms require a transition to “multicellular agency” that subsumes the agency of individual cells. Individual cognitive cells must integrate their sensory and metabolic processes, sharing bioelectric and biochemical information to form a macro-scale “self.” In this view, the development of a complex body is essentially a form of collective intelligence. The emergence of specialized cells - and eventually the nervous system - was not the invention of cognition, but a morphological scaling-up of the basal cognition already present in the single cell. The brain is simply a specialized organ that scaled the electrical excitability and communicative prowess that single eukaryotic cells already possess (Levin, 2019).
Rethinking Artificial Intelligence and Information
These three pillars all come together in understanding the cognitive cell (Lyon, 2015) as the fundamental unit of intelligence. Looking at the cell through a cognitive lens, and treating the cell as an active cognitive device, are interrelated projects that have implications regarding the relationship between the physical and the informational aspects of life. It reveals how thermal noise, chemical gradients, and physical forces are translated into biological meaning.
Furthermore, exploring these cellular architectures offers the possibility of technological applications. Today, the field of Artificial Intelligence is overwhelmingly dominated by artificial neural networks - architectures inspired by the human brain. But if we recognize that single cells have been expertly processing information, learning from their environments, and optimizing complex routing problems for billions of years without synapses, we open the door to entirely new paradigms. By studying cognition in the cellular world, we might be able to design new forms of artificial intelligence and bio-inspired computing whose architectures are more efficient, resilient, and different from anything we are currently investigating.
BTW, it’s not that our ideas of cognition will enter the cellular realm unscathed; it may well turn out that the features we consider to be ‘marks of the mental,’ aren’t universal, but rather, tied to the demands of the macroscopic world we inhabit. For example, we don’t need to spend cognitive cycles on finding oxygen because its concentration doesn’t vary much at our scale, but not so for a unicellular organism, where oxygen might vary quite a bit at the scale of, say, a hundred body lengths. Perhaps the essential features of cognition and subjectivity such as perception, memory, intentionality, selfhood, consciousness etc, are tied to the ecological scale we inhabit, that meter long organisms have a very different lifeworld (or Umwelt, as termed by the pioneering biosemioticist Jakob von Uexkull (Uexkull, 2013)) from nanometer long organisms.
> There’s no reason to assume that memory or attention or selfhood remains the same at the scale of a bacterium as they do for us even if bacteria possess some version of those features.
Why Should a Microbiologist Care?
The history of microbiology tells us that it is a folly to think of microbes as “simple” creatures. At this moment in time, microbial cognition may not be as far fetched an idea with many documented examples of learning-like behaviour (Messer et. al., 2026). Modern techniques are making it possible to study single-cell behaviour in real time. Perhaps, the time is ripe for an integrated theoretical and experimental approach to microbial cognition.
We have made a lot of progress by identifying molecular mechanisms behind microbial phenomena: molecule A phosphorylates molecule B, which regulates a gene C. That approach has been indispensable for mapping the cell’s hardware and elucidating particular systems. The molecular approach, when carried out quantitatively, has informed our understanding of robustness and fidelity of signalling. A cognitive lens might be a natural generalization of the quantitative-molecular approach. David Marr’s approach to vision (Marr, 2010) is our guide here - we need computational theory, not just biological implementation.
The cognitive lens could also work as a kind of ecological Rosetta Stone. In the lab we can switch specific pathways on and off, but we often have no idea what those signals actually mean to the cell out in the wild. Treat the cell as an agent that values resources and anticipates threats, and its internal circuitry becomes a way to reverse-engineer the ecology it evolved in: what it bothers to compute tells you the typical environment it encounters in the wild - an extension of reverse ecology (Levy and Borenstein, 2012).
We aren’t asking you to forget biochemistry, but to recognize - again in a David Marr-ian mode - that there are other levels of description. Separating the levels sharpens the questions we ask at each level. The biochemical level might ask “what does this protein do?” while the computational level might ask “what problem is this cell solving?”, and that second question opens up experiments that the chemical perspective misses: tests for memory, habituation, even associative learning.
Conclusion
The project of Cellosophy invites us into a bottom-up, biogenic perspective on intelligence. By studying the behaviors of ciliates, slime molds, and bacteria, we learn that nature has been ‘thinking’ for a very long time. Cognition is an evolved biological trait, as ancient and essential as metabolism. It represents the organism’s ongoing effort to bridge the chaotic external world with the delicate internal equilibrium required for survival.
Ultimately, Cellosophy challenges us to look through the microscope not just to see the mechanics of life, but to witness the primordial origins of the mind. The single cell is not a biological machine; it is a biological agent (Ball, 2026). And by studying it, we may finally come to understand the unbroken continuum of intelligence that unites every living creature on Earth.
A final word about the logistics of this newsletter: we hope to write a fresh essay once every few weeks. During the initial exploratory stage, our coverage will vary a lot, from theoretical issues to experimental findings and everything in the middle; but the goal is to turn this exploration into a research program by identifying researchable questions that can be tested in the lab and models that can be used to predict experimental outcomes as well as drive technological developments.
References
Arnellos, A., & Moreno, A. (2016). Integrating constitution and interaction in the transition from unicellular to multicellular organisms. Multicellularity. Origins and evolution, 249-275.
Ball, P. (2026). Is Life Just Different? Quanta Magazine. https://www.quantamagazine.org/is-life-just-different-20260708/
Baluška, F. (2025). Cognitive Cells: From Cellular Senomic Spheres to Earth’s Biosphere. Biosemiotics / Biol Theory.
Beniaguev, D., Segev, I., & London, M. (2021). Single cortical neurons as deep artificial neural networks. Neuron, 109(17), 2727–2739.e3. https://doi.org/10.1016/j.neuron.2021.07.002
Dexter, J., Prabakaran, S., & Gunawardena, J. (2019). A Complex Hierarchy of Avoidance Behaviors in a Single-Cell Eukaryote. Current Biology, 29, 4323–4329.e2.
Gidon, A., Zolnik, T. A., Fidzinski, P., Bolduan, F., Papoutsi, A., Poirazi, P., Holtkamp, M., Vida, I., & Larkum, M. E. (2020). Dendritic action potentials and computation in human layer 2/3 cortical neurons. Science, 367(6473), 83–87. https://doi.org/10.1126/science.aax6239
Jennings, H. S. (1906). Behavior of the lower organisms (No. 10). Columbia University Press, The Macmillan Company.
Levin, M. (2019). The Computational Boundary of a “Self”: Developmental Bioelectricity Drives Multicellularity and Scale-Free Cognition. Frontiers in Psychology.
Levin, M., & Dennett, D. (2025). Cognition all the Way Down. Aeon. https://aeon.co/essays/how-to-understand-cells-tissues-and-organisms-as-agents-with-agendas
Levy, R., & Borenstein, E. (2012). Reverse ecology: from systems to environments and back. In Evolutionary systems biology (pp. 329-345). New York, NY: Springer New York.
Lyon, P., & Cheng, K. (2023). Basal cognition: shifting the center of gravity (again). Animal Cognition, 26, 1743–1750.
Marr, D. (2010). Vision: A computational investigation into the human representation and processing of visual information. MIT Press.
Maturana, H. R., & Varela, F. J. (2012). Autopoiesis and cognition: The realization of the living. Springer Science & Business Media.
McCulloch, W. S., & Pitts, W. (1943). A logical calculus of the ideas immanent in nervous activity. Bulletin of Mathematical Biophysics, 5, 115–133. https://doi.org/10.1007/BF02478259
Messer, A., Oña, L., & Kost, C. (2026). Cognition without brains? Learning and memory in microorganisms. Trends in Microbiology.
Nakagaki, T., Yamada, H., & Tóth, Á. (2000). Maze-solving by an amoeboid organism. Nature, 407, 470.
Picard, M., & McEwen, B. S. (2018). Psychological stress and mitochondria: A conceptual framework. Psychosomatic Medicine, 80(2), 126–140. https://doi.org/10.1097/PSY.0000000000000544
Picard, M., & Shirihai, O. S. (2022). Mitochondrial signal transduction. Cell Metabolism, 34(11), 1620–1653. https://doi.org/10.1016/j.cmet.2022.10.008
Quian Quiroga, R., Reddy, L., Kreiman, G., Koch, C., & Fried, I. (2005). Invariant visual representation by single neurons in the human brain. Nature, 435, 1102–1107. https://doi.org/10.1038/nature03687
Ramanathan, S., & Broach, J. R. (2007). Do cells think?. Cellular and Molecular Life Sciences, 64(14), 1801–1804.
Ramón y Cajal, S. (1906). The structure and connexions of neurons [Nobel Lecture]. NobelPrize.org.
Rosenblatt, F. (1958). The perceptron: A probabilistic model for information storage and organization in the brain. Psychological Review, 65(6), 386–408. https://doi.org/10.1037/h0042519
Stuart, G. J., & Spruston, N. (2015). Dendritic integration: 60 years of progress. Nature Neuroscience, 18, 1713–1721. https://doi.org/10.1038/nn.4157
Thompson, E. (2010). Mind in life: Biology, phenomenology, and the sciences of mind. Harvard University Press.
Turing, A. M. (1937). On computable numbers, with an application to the Entscheidungsproblem. Proceedings of the London Mathematical Society, Series 2, 42(1), 230–265. https://doi.org/10.1112/plms/s2-42.1.230
Von Uexküll, J. (2013). A foray into the worlds of animals and humans: With a theory of meaning (Vol. 12). University of Minnesota Press.
Zhu, L., Kim, S.-J., Hara, M., & Aono, M. (2018). Remarkable problem-solving ability of unicellular amoeboid organism and its mechanism. Royal Society Open Science, 5(12).